
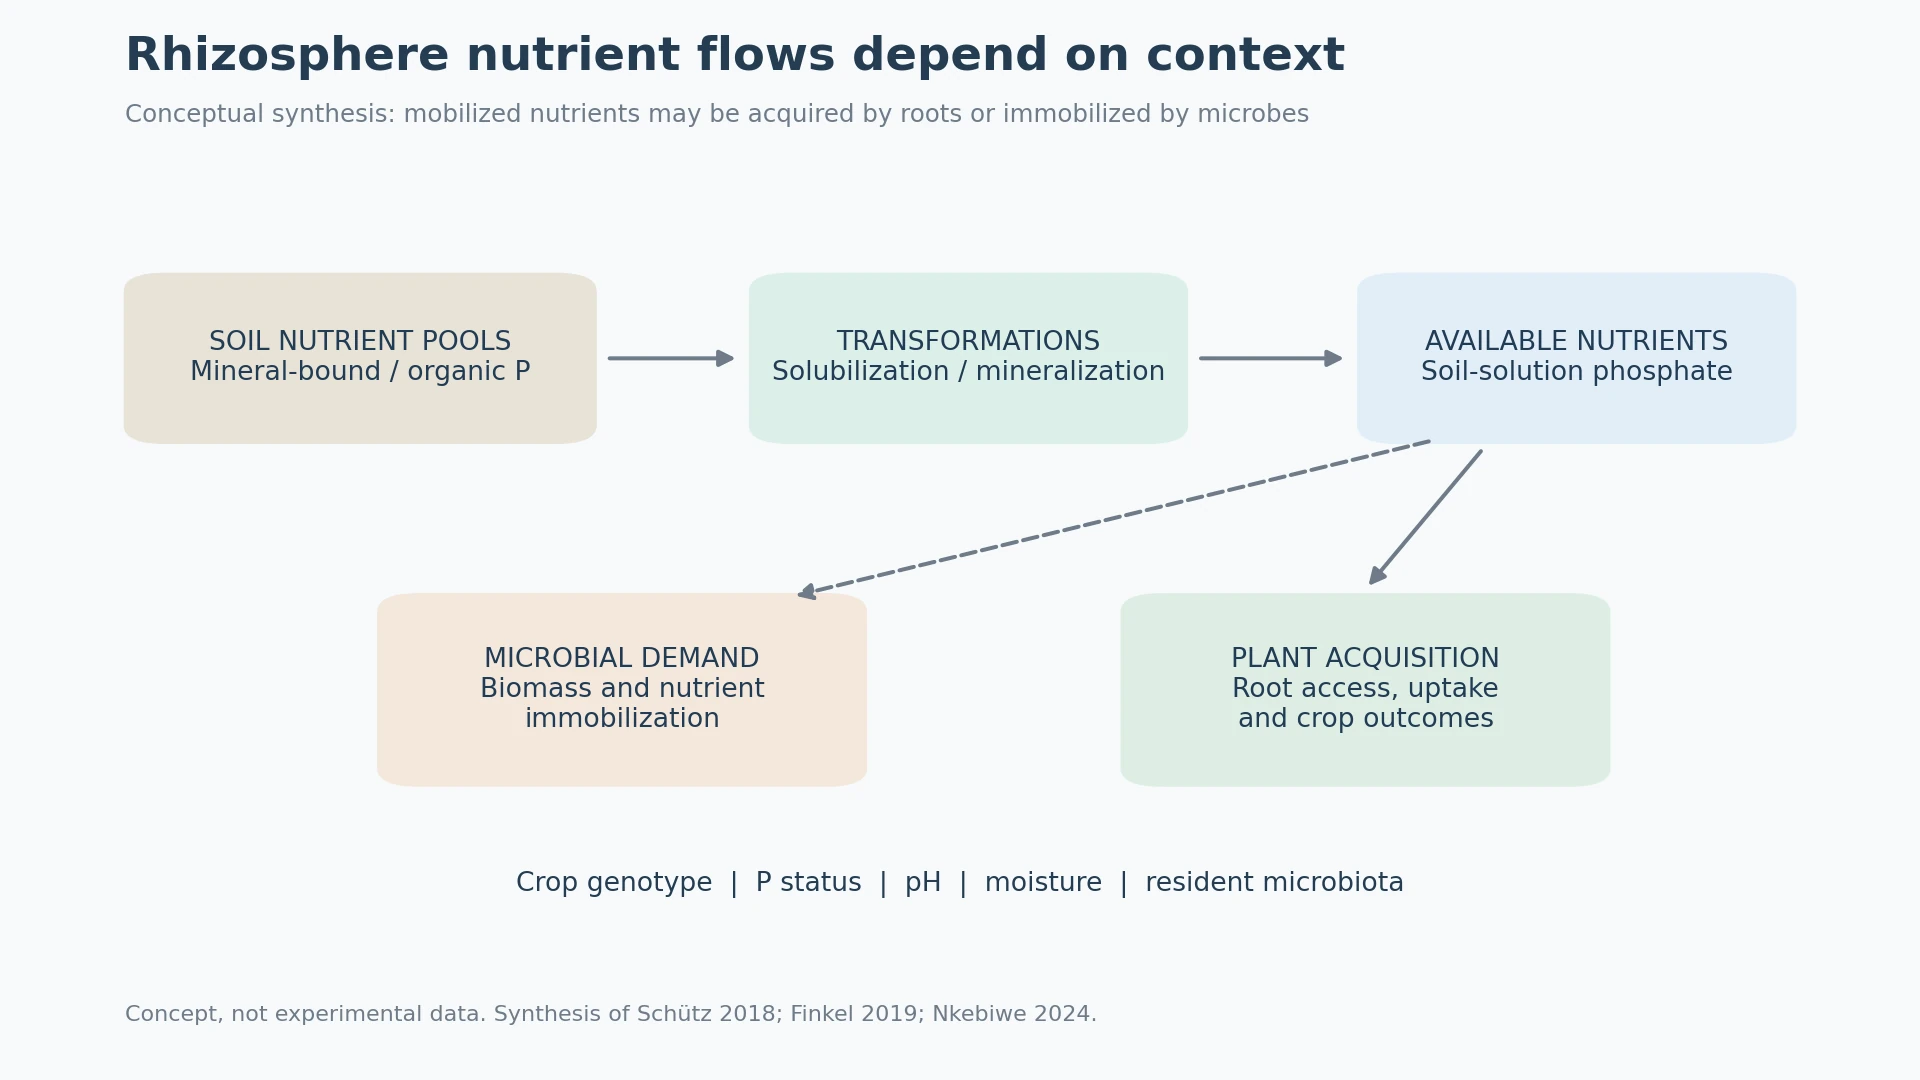
Rhizosphere microbes participate in nutrient transformations and may alter plant nutrient acquisition, but outcomes depend on the crop, soil, microbial material and management setting. Phosphate solubilization in culture, plant tissue phosphorus and field yield answer different questions. Research includes positive average responses to biofertilizers, nonsignificant field subgroups and nutrient competition between microbes and plants under low phosphorus. Understanding these differences turns a broad claim about root health into an agronomic question that can be measured and compared.[1, 2, 3]
A nutrient can be present without being accessible to roots
The rhizosphere is the soil interface influenced by root activity. Plants supply carbon, while microbes participate in nutrient transformations and community interactions. Soil phosphorus can bind to mineral surfaces, form poorly soluble compounds or occur in organic matter. Root exploration, water and soil chemistry also influence access. A soil with substantial total phosphorus therefore does not necessarily supply enough absorbable phosphorus at a particular time.[1, 3]
Phosphate solubilization and organic-phosphorus mineralization should not be treated as identical processes. The former mobilizes poorly soluble inorganic forms; the latter converts organic phosphorus into available forms. A microbial laboratory trait is a screening lead. Demonstrating plant benefit still requires nutrient uptake, biomass or harvested-yield measurements. Microbes consume resources themselves, so nutrient mobilization and greater plant acquisition are separated by an ecological relationship that needs testing.[1, 2, 3]
Under low phosphorus, microbes are not always helpers
Finkel and colleagues used Arabidopsis and phosphate-starvation-response mutants to examine how host responses and phosphorus availability jointly shape plant microbiota. They reconstructed interactions using a synthetic community of 185 bacterial isolates across phosphorus conditions. Effects on rosette size shifted from neutral or favourable to unfavourable. The plant phosphate-starvation response therefore changes the context of microbial interactions rather than simply reflecting soil nutrient supply.[2]
Under phosphate starvation, removing Burkholderia members from the community increased shoot inorganic-phosphate accumulation relative to the complete community. This supports competition for phosphorus by particular community members. It does not classify an entire genus as harmful or establish a universal commercial-crop response. Instead, it shows why community function must be interpreted in its host and nutrient context. More microbial species or a higher inoculation level does not itself guarantee greater nutrient acquisition.[2]
Global evidence supports potential, with important context dependence
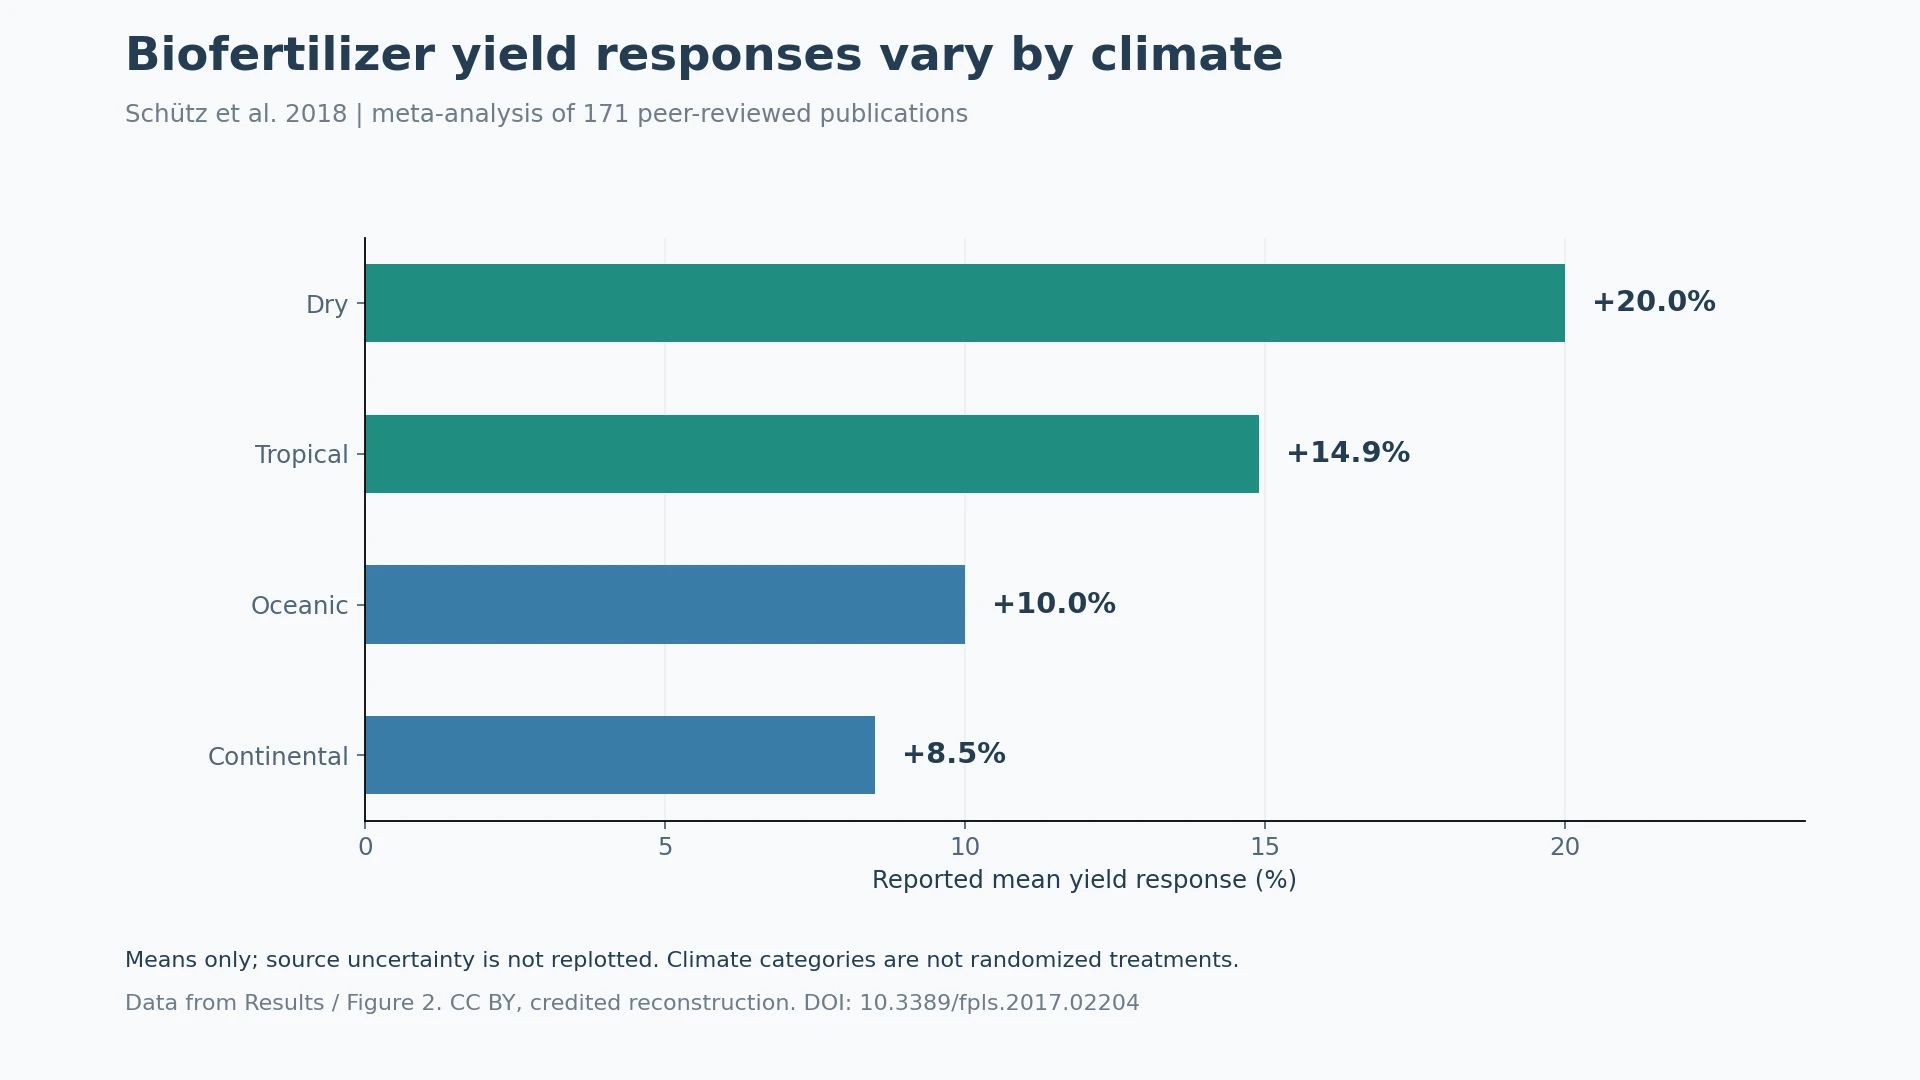
Schütz and colleagues combined 171 eligible peer-reviewed publications to examine biofertilizer responses in crop yield and nitrogen and phosphorus use. Average yield response across crops was +16.2%, but climate-group means differed: +20.0% in dry climates, +14.9% in tropical climates, +10.0% in oceanic climates and +8.5% in continental climates. These are averages across included studies, not an expected yield increase for a particular strain or product at every site.[1]
Even within the dry-climate category, 45% of comparisons involved irrigation. A climate label is consequently not equivalent to an experimental drought treatment. Phosphate-solubilizing organisms, nitrogen fixers and mycorrhizal fungi also represent different functions, while soil phosphorus methods and management backgrounds vary. Cross-study averages help establish direction; selecting a material still requires checking whether crops, strains, soils and fertilization backgrounds are comparable.[1]
| Study | Material and context | Main interpretation |
|---|---|---|
| Schütz 2018 | Cross-crop biofertilizer meta-analysis | Positive average responses with different climates, materials and soils.[1] |
| Finkel 2019 | Arabidopsis; 185-member bacterial community | Low phosphorus can favour competition rather than promotion.[2] |
| Nkebiwe 2024 | Microbial/non-microbial bio-effectors; pot and field trials | Field subgroup nonsignificant; the pooled 9.3% is not exclusively microbial.[3] |
Why controlled-environment responses can weaken in the field
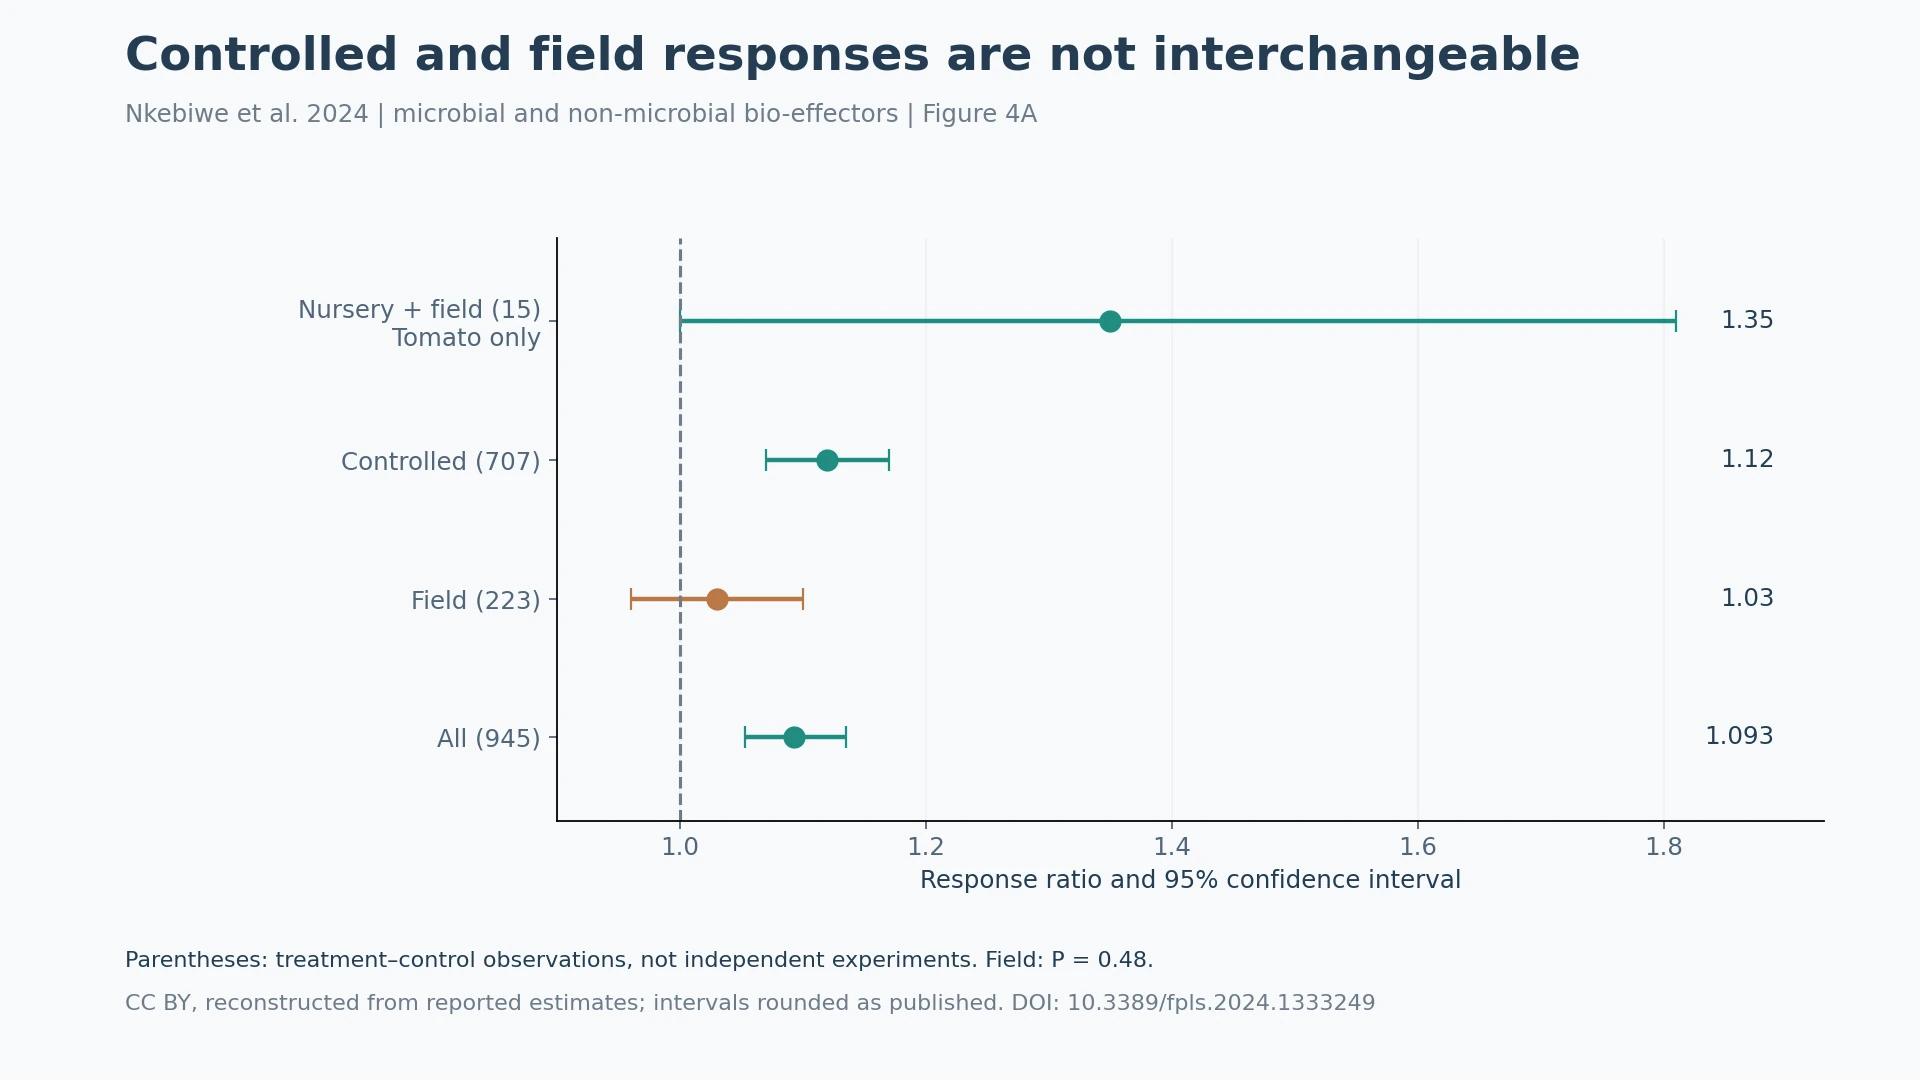
Nkebiwe and colleagues analysed BIOFECTOR experiments from Europe and Israel in 2024. Materials included microbial and non-microbial bio-effectors. Of 141 original experiments, 136 met the basic eligibility criteria. The main production analysis contained 945 treatment–control observations from 114 experiments, arranged in 290 shared-control clusters to address dependence. These counts refer to data pairs and experiments, not 945 individual plants or 945 independent field trials.[3]
The overall response ratio was 1.093, equivalent to an average increase of 9.3%. By growing condition, the controlled subgroup had a ratio of 1.12 with a 95% confidence interval of 1.07–1.17. The direct-field subgroup had a ratio of 1.03, with a 95% interval of 0.96–1.10 and P=0.48, which was not significant. The nursery-to-field category had a larger response but included only tomato, preventing attribution of the difference entirely to nursery management. Because materials were not exclusively microbial, the pooled result is not a pure microbial-inoculant effect.[3]
The same analysis found a positive overall response in above-ground phosphorus content, whereas the overall root-biomass response was not significant, with P=0.079. Nutrient, root and harvest endpoints therefore need not move together. Field rooting volume, resident-community competition, soil moisture and conditions for establishment may affect translation from laboratory function to agronomic performance. Comparable crops and materials need direct evaluation; a root photograph alone cannot establish a yield benefit.[3]
Connect rhizosphere functions to agronomic value with three measurement sets
First, record the environmental background: soil pH, the available-phosphorus method, organic matter, salinity, moisture and baseline fertilizer inputs. Second, measure plant responses: root traits, biomass, tissue nutrient concentrations and total nutrient uptake. Concentration and total uptake are different quantities. Greater biomass may dilute a concentration, so a leaf nutrient percentage alone is insufficient. Third, assess harvest yield, quality and input costs, with controls, replication and a defined observation period.[1, 3]
A fertilizer-reduction claim needs direct comparisons of conventional fertilization, reduced fertilization and reduced fertilization with the tested material, together with maintenance of yield and quality. Greater nutrient uptake at the same fertilizer level does not establish a particular fertilizer-saving percentage. Microbial tools are most useful when matched with soil diagnosis, balanced nutrition and water management so that a measurable function can operate in a defined setting.[1, 3]
| Objective | Measurements to combine | Insufficient alone |
|---|---|---|
| Improve phosphorus use | Soil-P method, total plant uptake and biomass | A solubilization halo in culture |
| Improve roots | Root traits, biomass, establishment and soil context | One root photograph or a taxon proportion |
| Reduce fertilizer inputs | Reduced/conventional fertilizer controls, yield, quality and costs | A higher nutrient concentration at unchanged fertilizer input |
Move from functional leads to reproducible crop outcomes
There is a biologically meaningful relationship between rhizosphere microbes and nutrient use, but it is not unconditional mutualism. Laboratory solubilization assays identify candidate functions, host–community studies explain potential competition, and multi-site or field evidence determines the scope of agronomic claims. The useful basis for evaluating a microbial strategy is a traceable connection between material identity, soil conditions, plant acquisition and harvested outcomes, rather than a general growth-promotion label.[1, 2, 3]
References
[1] Schütz L, Gattinger A, Meier M, et al. (2018). Improving Crop Yield and Nutrient Use Efficiency via Biofertilization—A Global Meta-analysis. Frontiers in Plant Science, 8:2204. DOI: 10.3389/fpls.2017.02204.
[2] Finkel OM, Salas-González I, Castrillo G, et al. (2019). The effects of soil phosphorus content on plant microbiota are driven by the plant phosphate starvation response. PLOS Biology, 17(11):e3000534. DOI: 10.1371/journal.pbio.3000534.
[3] Nkebiwe PM, Stevens Lekfeldt JD, Symanczik S, et al. (2024). Effectiveness of bio-effectors on maize, wheat and tomato performance and phosphorus acquisition from greenhouse to field scales in Europe and Israel: a meta-analysis. Frontiers in Plant Science, 15:1333249. DOI: 10.3389/fpls.2024.1333249.
This article supports scientific interpretation and does not establish efficacy for a particular commercial product or production site.